Current research review · 12 October 2026
Nuclear Microrheology: Measuring Local Response in a Living Composite
From fluorescent tracers to calibrated forces and frequency-dependent mechanics
Download the matching Word reviewAbstract
Nuclear microrheology asks how a small part of the nuclear interior moves or deforms on a specified length and time scale. It connects molecular mobility, chromatin organization and material response, but these connections depend on the probe and the model. Thermal particle motion, fluorescent-protein diffusion, targeted magnetic twisting and indentation of the nuclear surface are different experiments. Recent work combines these approaches with chromatin imaging, metabolic perturbation and comparisons between live and isolated nuclei. The resulting picture is a mechanically heterogeneous, active composite whose response cannot be represented adequately by one universal nuclear viscosity or stiffness. [1] [2] [3] [4] [5]
This review develops the physical inference framework before comparing experimental results. It emphasizes probe coupling, spatial sampling, the distinction between transport and stress response, and the biological state of the preparation. Studies published in 2024–2025 strengthen direct force-based measurements while also showing why isolation, metabolic activity and observation frequency change the answer. These findings support a more precise account of nuclear material behavior rather than a categorical claim that every nuclear component is a liquid, gel or solid. [6] [3] [4] [5]
1. Define the material question before choosing the probe
The nucleus presents at least three linked physical questions. A soluble protein searches through an accessible fluid and exchanges with binding sites. A chromatin locus moves while remaining part of an extended polymer and interacting network. An imposed deformation loads that network together with its boundary. A measurement can be informative about one of these questions without identifying the others. Inert GFP oligomer measurements, for example, characterize mobility through sampled nuclear regions; stretching an isolated nucleus interrogates resistance transmitted across a much larger structure. Treating both results as interchangeable measures of viscosity loses the physical distinction that gives them meaning. [2] [7] [8]
Microrheology is local because the probe interrogates the material to which it couples, over distances and times accessible to the experiment. Locality is not guaranteed merely by using a small fluorescent object. A small object may bind to an extended structure, encounter a boundary or report active displacement. Conversely, a surface indentation involves a spatial stress field that can recruit components outside the apparent contact point. A useful account therefore specifies probe size, surface chemistry, position, imposed load, observation frequency and nuclear preparation before interpreting a numerical result. These specifications define the material comparison, rather than serving as optional technical annotations. [9] [3] [4]
2. Passive motion and the thermal inference problem
In passive particle microrheology, trajectories are observed without an externally imposed test force. For ideal Brownian translation in d observed dimensions, the mean squared displacement is 2dDτ, where D is a diffusion coefficient and τ a lag time. In a dilute Newtonian fluid, the Stokes–Einstein relation D = kBT/(6πηa) connects diffusion to viscosity η for a spherical probe of hydrodynamic radius a with the assumed boundary condition. The units matter: D has dimensions of length squared per time, whereas η is measured in Pa·s. Converting between them already assumes a physical model and known probe coupling. [1] [9] [10]
A generalized relation can connect thermal displacement statistics to linear viscoelastic response, extending the analysis beyond a single Newtonian viscosity. Its usefulness does not make every cellular trajectory a valid rheometer. The fluctuation-based inference requires an appropriate continuum description, coupling between probe and material, and a regime in which measured fluctuations represent the assumed thermal response. Directed activity, binding, finite accessible spaces and heterogeneous environments can change trajectory statistics. Subdiffusion therefore identifies a departure from simple unrestricted Brownian motion; it does not by itself identify one molecular mechanism or uniquely determine the elastic modulus of chromatin. [1] [9] [7] [11]
3. Fluorescent mobility measurements complement rheology
Fluorescence correlation spectroscopy measures fluctuations in a calibrated observation volume. Dross and colleagues studied eGFP oligomers in living nuclei outside nucleoli and fitted their correlation data with two normally diffusing fluorescent components plus a triplet-state contribution. Calibration and optical geometry were integral to the calculation. These observations establish probe-dependent mobility in the regions sampled by that experiment. They do not show that an arbitrary DNA-binding protein should have the same mobility, or that two fitted components correspond uniquely to two physically separate fluid phases. Probe chemistry and the observation model remain part of the result. [2]
Single-particle tracking follows labeled molecules and can expose heterogeneity concealed by an average. The Spot-On study demonstrated that motion blur, loss of rapidly moving molecules from the focal volume, localization uncertainty and excessive particle density can bias estimated populations. Its model uses steady-state Brownian subpopulations with acquisition corrections. These are explicit assumptions, not a direct movie of all molecular states. For nuclear microrheology, a trajectory analysis should distinguish freely moving, transiently bound and persistently constrained probes before a change in apparent diffusion is assigned to material resistance. Otherwise, a change in occupancy may be misread as a change in viscosity. [11] [12]
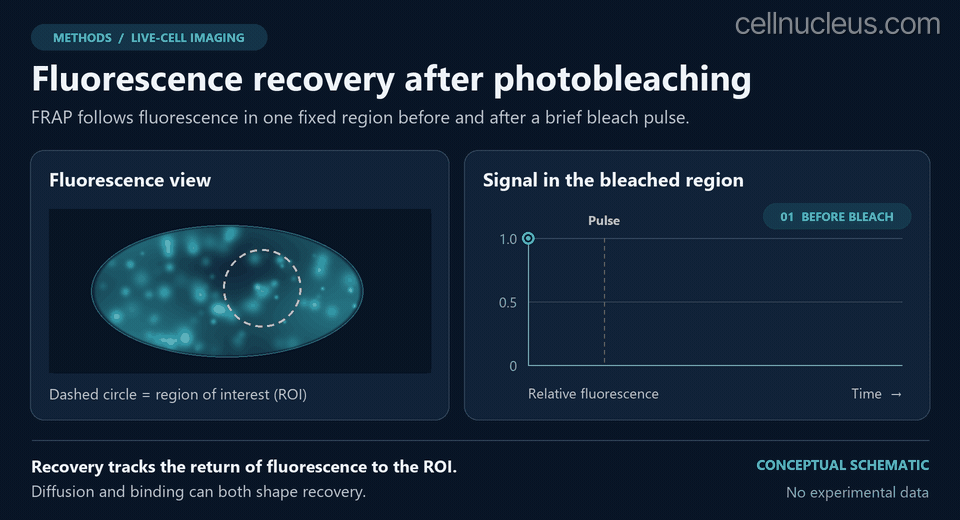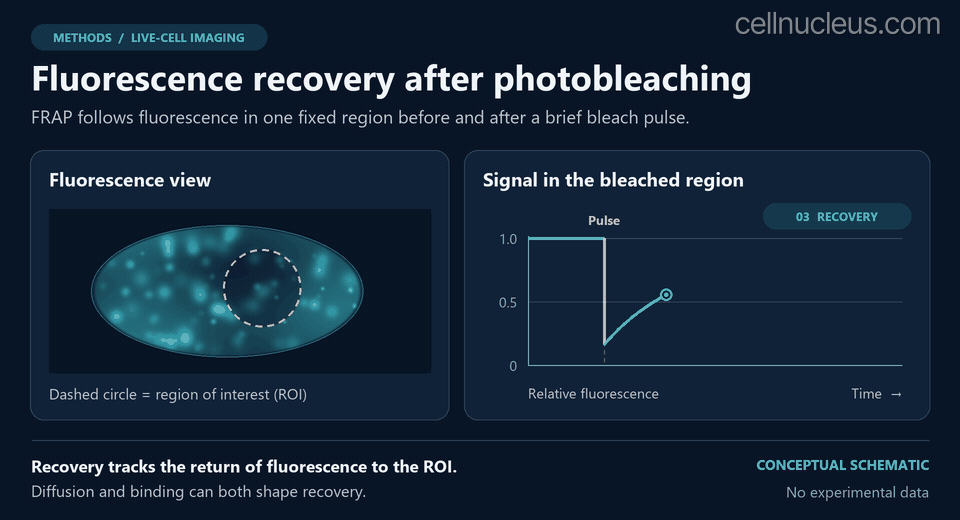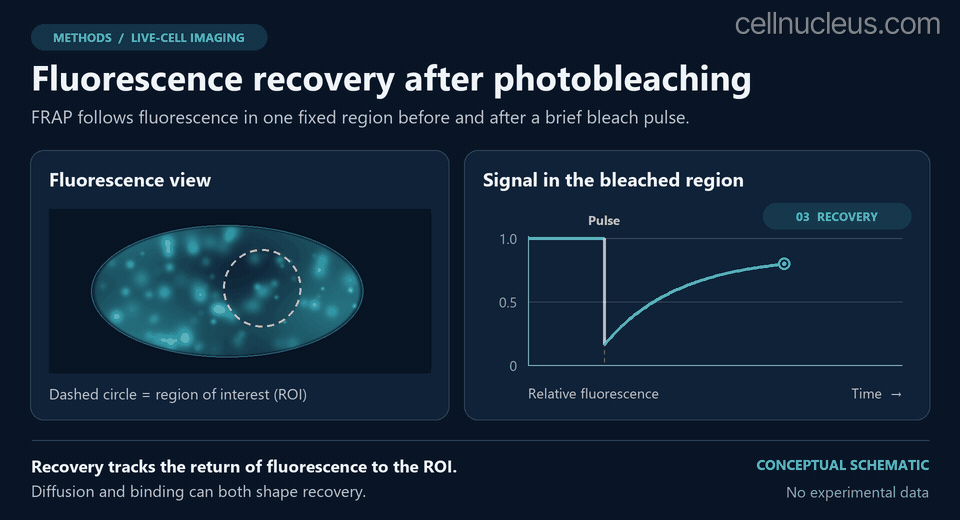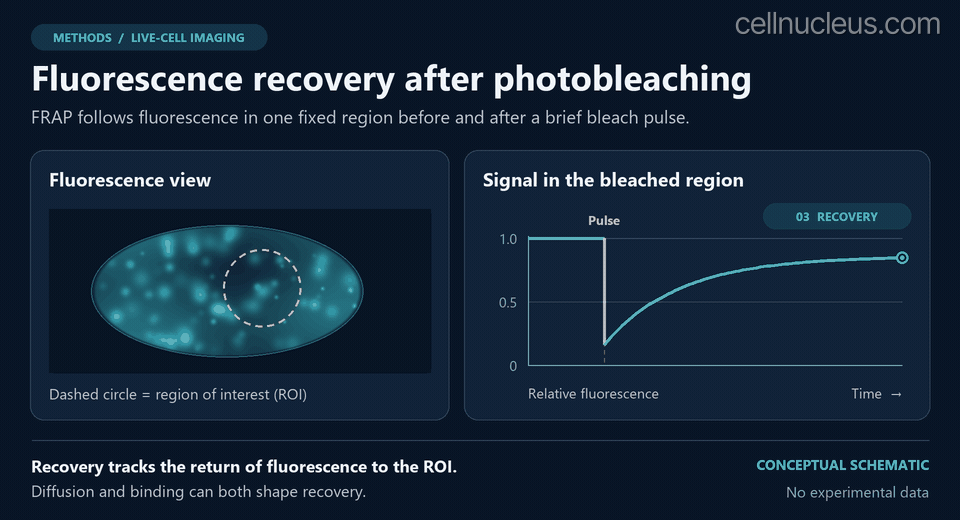
FRAP supplies another complementary observable: recovery of fluorescence after bleaching a region. Reaction–diffusion analysis can separate some contributions of transport and binding when the experiment and model contain enough information. Sprague and colleagues showed why recovery analysis requires considering both processes and their limiting regimes. A recovery half-time alone is not an intrinsic viscosity, and a recovered fluorescent fraction is not a direct mechanical loss modulus. Changing the size or position of the bleached region can help test the interpretation, but the chosen model still determines which kinetic parameters are identifiable. [13]
Show the fluorescence recovery animation
4. Active probes test force transmission
Active microrheology applies a calibrated force or torque and measures the resulting displacement or deformation. It directly asks how the sampled structure responds, rather than inferring response solely from spontaneous fluctuations. In a sinusoidal experiment, the phase difference between applied stress and measured strain separates an in-phase storage contribution from an out-of-phase loss contribution. Their relative magnitudes depend on frequency. The experiment also depends on how stress reaches the material: an antibody-bound nanoparticle and an uncoated particle need not load the same nuclear structure even when their nominal diameters are similar. [9] [3]
Rashid and colleagues used approximately 200-nm-diameter ferromagnetic particles in living nuclei. Anti-H2B coating targeted chromatin, whereas uncoated and control-coated particles supplied different coupling conditions. In the CHO reporter system, force-dependent chromatin deformation and frequency-dependent response were examined over 0.1–5 Hz. The study connected this local mechanical perturbation to persistent changes in mobility and transcriptional readouts, with a separate induced-pluripotent-stem-cell arm used for labeled RNA polymerase II. Those distinctions are essential: targeted chromatin loading, a local nucleoplasmic measurement and polymerase behavior are related observations, rather than one universal material constant. [3]
5. Whole-nucleus deformation supplies a different scale
Experiments on isolated nuclei establish that resistance changes with the amount and geometry of deformation. Stephens and colleagues distinguished chromatin-dominated response at smaller extensions from lamin-A-dependent strain stiffening at larger extensions. Bergamaschi and colleagues subsequently combined optical-tweezer force measurements with chromatin and boundary imaging and interpreted heterogeneous force response using a hierarchical chain model. Such measurements help assign load-bearing roles to components of the composite. A spring constant obtained from force versus extension nevertheless remains specific to the geometry; it cannot be substituted directly for a shear modulus or a viscosity without an additional mechanical model. [8] [6]
The coupling between chromatin and the boundary is itself mechanically consequential. Attar and colleagues used polymer modeling constrained by nuclear measurements to examine how peripheral tethering permits force applied at the lamina to recruit internal chromatin resistance. Their conclusion concerns load transmission in the specified model, rather than proof that every genomic region at the periphery forms a permanent mechanical attachment. This distinction explains why local mobility, chromatin compaction and global force response may change together in some perturbations and diverge in others: the coupling architecture can change alongside the material being loaded. [14] [8]
6. Frequency and preparation are biological variables
The 2025 AFM study by Pørtner and colleagues compared isolated and live MCF7 nuclei using an oscillating cantilever and frequency-dependent mechanical analysis. The modulus curves showed similar trends with a scaling difference, while the loss tangent disclosed more detailed differences between preparations. Actin depolymerization changed aspects of the low-frequency response, and a Jeffreys model described the measured spectra better than the alternative circuit compared in the study. These results show why one fitted elastic value is an incomplete description. The biological preparation and the rate of loading can alter how energy is stored and dissipated. [4]
Isolation has experimental advantages because it reduces some cytoplasmic and cytoskeletal contributions. It also changes the system under investigation. Buffer conditions, boundary support, membrane continuity and metabolic state can differ from those of the living cell. The MCF7 comparison does not establish that all isolated nuclei are uniformly softer or that any one preparation faithfully reproduces every live-cell response. It demonstrates that matching the cell system and examining an entire frequency spectrum can reveal differences that a single-rate assay would miss. Generalizations to another lineage, isolation protocol or loading geometry need their own matched comparison. [4] [5]
7. Nuclear activity can alter dissipation
Byfield and colleagues examined metabolically active karyoplasts, which retain an intact nucleus within a plasma-membrane-enclosed preparation rather than constituting bare detergent-isolated nuclei. Their compression experiments showed substantial dissipation and implicated chromatin-remodeling activity in the ability to undergo large reversible deformations. Inhibition with BRM-014 increased resistance and reduced dissipation. Because that compound acts on both BRM and BRG1, the pharmacological result should be described with its target scope even though the paper develops a BRG1-centered interpretation. The work supports an active contribution to mechanical behavior; it does not justify treating all dissipation as a passive viscous dashpot. [5]
The force-cessation experiments of Rashid and colleagues address a different aspect of activity: persistence after a transient perturbation. Mobility and polymerase-associated readouts remained changed for minutes after targeted chromatin loading ended. Such mechanomemory is longer than the immediate oscillatory response measured during loading and cannot be collapsed into the same relaxation time without further evidence. A complete experiment should distinguish rapid force response, recovery after release and delayed regulatory changes. These timescales connect mechanics to nuclear function while preserving the distinction between material relaxation and biological adaptation. [3] [5]
8. A nucleolar example anchors the units and context
Feric and colleagues demonstrated coexisting nucleolar subcompartments and studied reconstituted protein droplets separately from living nucleoli. In their in-vitro microrheology, tracer particles had a radius of 50 nm. NPM1 droplets showed approximately diffusive tracer motion and a reported viscosity of 0.74 ± 0.06 Pa·s under those preparation and analysis conditions; FIB1 droplets showed more pronounced subdiffusion. These particles were material probes inside purified droplets, rather than NPM1 molecules tracked across a whole living nucleus. The numerical result belongs to that particular component, preparation, probe and model. [10]
The same study also analyzed fusion dynamics in vivo, where the relevant fitted quantity included the ratio of viscosity to surface tension. That ratio has dimensions different from viscosity alone. A fusion relaxation time depends on both the object size and the restoring interfacial force, so importing a droplet coalescence time into a nuclear-viscosity table without the model would be misleading. The broader lesson is that rheology must retain the measured quantity, its units and the physical explanation linking the observation to a parameter. Similar-looking nuclear movies can encode different material information. [10] [9]
9. What each measurement can establish
| Approach | Direct observable | Supported interpretation | Main qualification |
|---|---|---|---|
| Inert-protein FCS | Fluctuation autocorrelation in a calibrated observation volume | Probe mobility and fitted populations in sampled regions | Binding, photophysics and optical geometry must be modeled [2] |
| Single-particle tracking | Displacement distributions and trajectory histories | Resolved mobility populations within acquisition limits | Fast-particle loss, blur, labeling and steady-state assumptions [11] |
| Targeted magnetic microrheology | Phase and deformation under applied torque | Local force response of the coupled chromatin or nucleoplasmic system | Coating, injection, geometry and perturbation define the sampled material [3] |
| Optical-tweezer nuclear stretching | Force–extension response with structural imaging | Component-dependent deformation and strain stiffening | Isolated preparation and chain-model interpretation [6] [8] |
| Oscillatory AFM | Contact-force phase and amplitude across frequency | Frequency-dependent modulus and loss tangent | Contact model, drag correction and live versus isolated preparation [4] |
| Compression of active karyoplasts | Loading/unloading work and shape response | Dissipation associated with metabolic and remodeling activity | Preparation differs from a bare nucleus; inhibitor target scope matters [5] |
The table suggests a practical strategy for interpreting a perturbation: measure more than one observable while keeping the biological state matched. A mobility change combined with altered binding populations favors a different account from a mobility change accompanied by a calibrated mechanical response. Concurrent imaging of chromatin and the nuclear boundary can determine which structure deforms, while a frequency sweep tests whether the perturbation affects storage, dissipation or both. Agreement between complementary measurements strengthens a material interpretation; agreement between two differently labeled estimates of the same fitted parameter is less informative when they share the same model assumptions. [11] [13] [6] [4]
10. A current synthesis and the next mechanistic questions
Current evidence supports treating the nucleus as a coupled, scale-dependent and active material. The strongest advances come from experiments that identify the loaded component, calibrate the force or optical volume, measure a time or frequency range, and preserve the distinction between in-vitro material and living-cell behavior. The remaining challenge is to connect those descriptions across scales: how local chromatin remodeling changes nuclear dissipation, how peripheral coupling recruits internal resistance, and when molecular transport can serve as a reporter of the same physical state. Answering these questions requires joint measurements rather than assuming that one diffusion coefficient predicts every mechanical response. [2] [14] [3] [4] [5]
References
- [1] Thomas G. Mason, David A. Weitz (1995). Optical Measurements of Frequency-Dependent Linear Viscoelastic Moduli of Complex Fluids. Physical Review Letters. 10.1103/PhysRevLett.74.1250
Evidence and source scope
Source type: primary. Access: Primary citation identity and primary abstract through author/index record; complete experimental text not read..
Thermal probe fluctuations related to linear viscoelastic response in tested complex fluids; extrapolation to actively driven nuclei requires additional assumptions.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [2] Nicolas Dross, Corentin Spriet, Monika Zwerger et al. (2009). Mapping eGFP Oligomer Mobility in Living Cell Nuclei. PLOS ONE. 10.1371/journal.pone.0005041
Evidence and source scope
Source type: primary. Access: Primary PLOS main Abstract, Methods data analysis/acquisition/calibration and selected Results/Discussion; no raw data reanalysis..
eGFP oligomer FCS outside nucleoli: calibrated two-normal-diffusion components plus triplet term; cell/model/probe constraints retained.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [3] Fazlur Rashid, Sadia Amin Kabbo, Ning Wang (2024). Mechanomemory of nucleoplasm and RNA polymerase II after chromatin stretching by a microinjected magnetic nanoparticle force. Cell Reports. 10.1016/j.celrep.2024.114462
Evidence and source scope
Source type: primary. Access: Primary manuscript main Summary, Results on microrheology and mechanomemory, Figures 1–5 and Discussion read; supplemental figures and raw measurements not reanalysed..
200-nm-diameter targeted magnetic particles in CHO DHFR reporter nuclei; 0.1–5 Hz force response and separate hiPSC Pol II arm; local perturbation and injection limitations.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [4] Ellen Juel Pørtner, Anna Mularski, Tobias William Jarrett, Stine Lauritzen Sønder, Jesper Nylandsted, Adam Cohen Simonsen (2025). Viscoelastic differences between isolated and live MCF7 cancer cell nuclei resolved with AFM microrheology. Journal of the Royal Society Interface. 10.1098/rsif.2024.0885
Evidence and source scope
Source type: primary. Access: Root independently read primary PMC12173521 Abstract and selected main Methods/Results paragraphs, including oscillatory preparation, hydrodynamic drag correction, morphology and Jeffreys analysis; primary Scite webpage identity corroborated. Supplement and raw-data reanalysis excluded..
Oscillatory AFM on live and isolated MCF7 nuclei, hydrodynamic-drag validation, modulus/loss-tangent distinction and Jeffreys model. The published author list supersedes incomplete Consensus authors.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [5] Fitzroy J. Byfield, Behnaz Eftekhari, Kaeli Kaymak-Loveless et al. (2025). Metabolically intact nuclei are fluidized by the activity of the chromatin remodeling motor BRG1. Biophysical Journal. 10.1016/j.bpj.2024.11.3322
Evidence and source scope
Source type: primary. Access: Published PDF front matter, main preparation/treatment Methods, Results around Figure 9 and Discussion read; supplementary data not appraised..
Metabolically active karyoplast compression/dissipation and BRM-014 inhibition; BRM-014 inhibits BRM and BRG1, so pharmacology is not exclusive genetic proof for BRG1. Karyoplasts are not bare detergent-isolated nuclei.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [6] G. Bergamaschi, A. Biebricher, Hannes Witt, F. Byfield, Xamanie M R Seymonson, Cornelis Storm, P. Janmey, G. Wuite (2024). Heterogeneous force response of chromatin in isolated nuclei.. Cell Reports. 10.1016/j.celrep.2024.114852
Evidence and source scope
Source type: primary. Access: Fetched Consensus primary abstract/record, cross-checked with SciSpace where available; complete body not appraised..
Bergamaschi and colleagues measured isolated-nucleus force responses together with chromatin and nuclear-envelope deformation. Chromatin was more compliant than the envelope below the reported 30% strain regime, and chromatin digestion softened nuclei. The joint readouts strengthen component interpretation in the tested preparation without defining one elastic modulus or viscosity for every nucleus. Bergamaschi et al. (2024) .
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [7] Fabian Erdel, Michael Baum, Karsten Rippe (2015). The viscoelastic properties of chromatin and the nucleoplasm revealed by scale-dependent protein mobility. Journal of Physics: Condensed Matter. 10.1088/0953-8984/27/6/064115
Evidence and source scope
Source type: primary. Access: Published identity and primary abstract from author-manuscript repository; full main text not appraised..
Differently sized inert GFP probes and polymer simulations; size-dependent intermediate-scale viscoelastic behavior and obstacle-network model; not universal fixed fractal organization.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [8] Andrew D. Stephens, Edward J. Banigan, Stephen A. Adam et al. (2017). Chromatin and lamin A determine two different mechanical response regimes of the cell nucleus. Molecular Biology of the Cell. 10.1091/mbc.E16-09-0653
Evidence and source scope
Source type: primary. Access: Primary abstract and bibliographic metadata; complete body unavailable through connector..
Chromatin and lamins contribute in separate isolated-nucleus extension regimes; spring constants are not universal moduli or viscosity.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [9] Todd M. Squires, Thomas G. Mason (2010). Fluid Mechanics of Microrheology. Annual Review of Fluid Mechanics. 10.1146/annurev-fluid-121108-145608
Evidence and source scope
Source type: seminal review. Access: Publisher bibliographic identity and abstract; established mathematical relationships independently checked dimensionally. Detailed review body not appraised..
Foundational synthesis of probe/bulk coupling, passive thermal-fluctuation and active-force microrheology assumptions; not a nuclear measurement.
No independent experimental replication or raw-data reanalysis. Source interpretation confined to the stated access depth.
- [10] Marina Feric, Nilesh Vaidya, Tyler S. Harmon et al. (2016). Coexisting Liquid Phases Underlie Nucleolar Subcompartments. Cell. 10.1016/j.cell.2016.04.047
Evidence and source scope
Source type: primary. Access: Primary main-text Results subsection on in-vitro viscoelasticity, Fig2E and main Experimental Procedures, independently checked in root browser; source detail received as collaborator evidence. No supplements/raw-data reanalysis..
Component-specific nucleolar coexistence and dynamics; in-vitro 50nm-radius tracer values belong to reconstituted NPM1/FIB1 droplets.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [11] Anders S. Hansen, Maxime Woringer, Jonathan B. Grimm et al. (2018). Robust model-based analysis of single-particle tracking experiments with Spot-On. eLife. 10.7554/eLife.33125
Evidence and source scope
Source type: primary. Access: Primary indexed main Introduction and selected Results/model/simulation evaluation, first8000char source excerpt; not complete article..
Spot-On model/testing distinguishes localization, defocalization, density and motion-blur biases with steady-state Brownian populations.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [12] Aurélien Bancaud, Sébastien Huet, Nathalie Daigle et al. (2009). Molecular crowding affects diffusion and binding of nuclear proteins in heterochromatin and reveals the fractal organization of chromatin. The EMBO Journal. 10.1038/emboj.2009.340
Evidence and source scope
Source type: primary. Access: Primary abstract and bibliographic metadata; complete body unavailable through connector..
Tracer exclusion/hindrance and transient chromatin-protein trapping; fractal interpretation remains model dependent.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [13] Brian L. Sprague, Robert L. Pego, Diana A. Stavreva et al. (2004). Analysis of Binding Reactions by Fluorescence Recovery after Photobleaching. Biophysical Journal. 10.1529/biophysj.103.026765
Evidence and source scope
Source type: primary. Access: Primary abstract and bibliographic metadata; complete body unavailable through connector..
Reaction-diffusion FRAP solutions constrain binding inference; not every recovery curve identifies every parameter.
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
- [14] A. G. Attar, J. Paturej, Ozan S. Sarıyer, E. Banigan, A. Erbaş (2025). Peripheral heterochromatin tethering is required for chromatin-based nuclear mechanical response. Nucleic Acids Research. 10.1093/nar/gkaf763
Evidence and source scope
Source type: primary. Access: Fetched Consensus primary abstract/record, cross-checked with SciSpace where available; complete body not appraised..
Attar and colleagues used polymer simulations compared with micromechanical and chromosome-contact measurements. In that model, peripheral chromatin attachment transmitted imposed nuclear forces to chromatin, and internal crosslinks stiffened the nucleus only when that peripheral coupling was present. This is a model-constrained account of load transfer; a mapped lamina association by itself does not establish the strength or permanence of every molecular tether. Attar et al. (2025) .
No indexed notice in retrieved result is not a guarantee of no correction/retraction. New records lacked complete Scite notice check after monthly quota.
Evidence scope
This review integrates published primary research with a foundational methods review where needed. Source access ranges from primary abstracts to the selected main Results and Methods identified in each reference record. It is a scholarly synthesis rather than an independent reanalysis of experimental data. Conclusions retain the biological system, measurement scale and model assumptions of the cited studies.